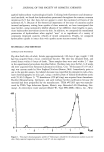
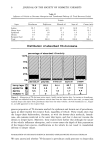
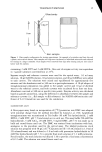
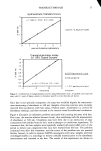
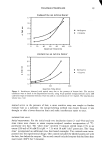
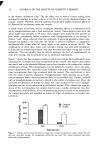
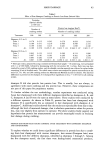
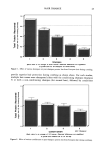
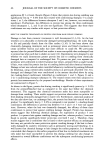
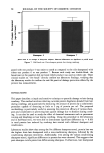
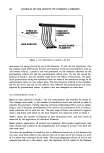
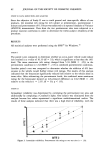
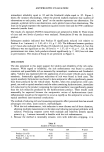
TRANSGLUTAMINASE 21 Table II Loss Of Enzyme Activity Following Incubation With Hair Enzyme activity Trial Conditions (% of control) 1 Control (no hair/no incubation) 100 2 No hair/2-hr incubation, 37øC 54 3 No hair/4-hr incubation, 37øC 50 4 With hair/2-hr incubation, 37øC 70 5 With hair/4-hr incubation, 37øC 63 into the hair during incubation, penetrating below the hair surface. In contrast, the enzyme's size limited covalent incorporation to the surface only, requiring isotope activity at the surface to be measurable above a "background" of non-specific binding inside the hair. Inasmuch as the number of potential non-specific binding sites inside the hair was orders of magnitude in excess of specific surface sites, a threefold strategy was adopted to decrease non-specific binding. First, after the normal wash and rinse preparation steps, hair samples were preincubated for 12 hours in either pure buffer (50 mM Tris-HCl, pH 7.5) or a buffered amine solution (50 mM Tris-HCl, 10 mM "cold" putrescine-HCl, pH 7.5) to saturate amine binding sites inside the hair. Second, the enzyme incubation time was reduced from 2-4 hours to only 30 minutes to limit diffusion. Third, post-incubation buffer rinses were added to remove non-covalently bound material. Three, 250-ml, 15-minute buffer rinses were used for all samples as a "short rinse." Half of the samples received an additional overnight soak in two more changes of buffer as a "long rinse." Trial incu- bations were done without enzyme to test the efficacy of the preincubation and rinsing procedures. Figure 6 shows the results of experiments with two rinse times and two preincubation treatments. For both amine- and buffer-preincubated samples, longer rinsing reduced non-specific binding to about 12% of shorter rinse-time values. Preincubation with the amine solution reduced non-specific binding by another factor of two. The overall amount of non-specific binding was also reduced in all experiments because of the use 12500 10000 7500 5000 2500 0 [] Short rinse [] Long rinse Buffer Amine Preincubation solution Figure 6. Effect of preincubation type and rinse length on non-specific binding. The hair was preincubated with either assay buffer (50 mM Tris-HCl, pH 7.5) or an amine buffer (50 mM Tris-HCl, 10 mM unlabeled putrescine-HC1, pH 7.5). The "short-rinse" used 250 ml soaks (3x) of buffer, for 15 minutes each. The "long rinse" consisted of an additional buffer change and soak overnight.

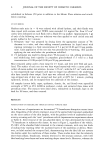
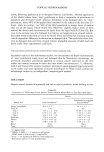
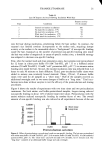
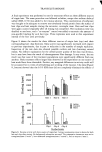
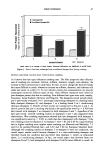
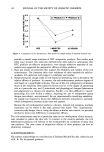
22 JOURNAL OF THE SOCIETY OF COSMETIC CHEMISTS of the shorter incubation time. The net effect was to reduce activity arising from non-specific binding to within a factor of 10-20 of the activity observed from a "no isotope" control. Therefore, the new conditions would allow smaller treatment effects to be observed for incubations using the enzyme. A single source of hair was used to investigate treatment effects in combination with active transglutaminase and a heat-inactivated control. Preincubation time with the amine buffer was extended to 20 hours. Hair samples were rinsed for five minutes in pure buffer immediately before incubation with transglutaminase in an attempt to remove "cold" amine substrate from the proximity of potential glutamine donor sites. Enzyme was added to the vials after the isotope to prevent hydrolysis, a competitive mechanism that occurs when an amine donor is not present in excess (40,41). The combination of three short rinses and overnight rinsing was used after incubation. Unlike previous isotope experiments, hair clips were also saved after rinsing and counted separately. This was initially done in order to ascertain the level of contamination on clips after rinsing, and for possible reuse in additional experiments. Figure 7 shows that hair samples incubated with active enzyme had significantly more incorporation of isotope than hair incubated with the control. The relative data scatter was small, and so the observed difference was at first thought to be evidence for covalent modification of hair. This interpretation was not definitive, however, due to the unex- pected observation that metal hair clips incubated with active enzyme also exhibited more incorporation than clips incubated with the control. This was believed to have been the result of protein adsorption. Transglutaminase itself functions as a poor glu- tamine substrate when a better glutamine donor is not available (42). Further, proteins such as transglutaminase are known to adsorb to the surface of stainless steel. Thus, the increased incorporation of isotope for metal hair clips incubated with active transglu- taminase was due to the adsorption of self-labeled enzyme. This clouded the interpre- tation of the corresponding hair sample data because a similar mechanism may have overwhelmed covalent effects. In lieu of determining the exact nature of the mechanism, the rinsing procedure was modified to reduce the effect of adsorption on further mea- surements. 1200 ,--, [] ConSol 1:• 900 [] AcUve t:zo 600 ,•..•. , ,,• '• 300 o H•r Clips Substrate Figure 7. Enzyme activity with one source of virgin hair. Isotope incorporation (cpm) is shown for both hair and clips after rinsing. No background subtraction was used. The control treatment used heat- denatured transglutaminase.
Purchased for the exclusive use of nofirst nolast (unknown)
From: SCC Media Library & Resource Center (library.scconline.org)